Characterizing Envelope Region Enhancer Activity in HIV-1
Arden Nasveschuk
Senior Thesis | 2026
CharacterizingEnvelopeRegionEnhancerActivityinHIV-1
ArdenNasveschuk
BostonUniversityAcademy
2March2026
Introduction
Humanimmunodeficiencyvirus(HIV),thecausative pathogenbehindacquiredimmunodeficiencysyndrome(AIDS), haspresentednumerousmedicalandpublichealthchallengessince itsdiscoveryinthe1980s.HIVtargetsimmunecells,weakening theimmunesystemandmakingindividualsmoresusceptibletoa varietyofinfections.Ifleftuntreated,HIVeventuallyprogressesto AIDS,aseriousconditiondefinedascoinfectionofHIVand anotherpathogen.AlthoughthereareeffectivetreatmentsforHIV, itistypicallyincurable.Furthermore,despiterecentadvancements inpreventingandtreatingHIV,theHIVepidemicisstillongoing; asof2024,thereare40.8millionpeoplelivingwithHIVglobally (JointUnitedNationsProgrammeonHIV/AIDS,n.d.).
Additionally,therewereapproximately1.3millionnewHIV infectionsin2024.HIV-relatedinfectionsanddeathsareexpected toincreaseinthecomingyearsduetotheshutdownoftheUnited States’foreignaidprogramsaddressingtheHIVepidemic, includingtheU.S.President’sEmergencyPlanforAIDSRelief (PEPFAR);theUnitedNationsestimatestherewillbe6.6million additionalHIVinfectionsand4.2millionadditionalAIDS-related deathsbetween2025and2029duetothelossofPEPFARand otheraidprograms(JointUnitedNationsProgrammeon HIV/AIDS,2025).Thisunderscorestheongoingseverityofthe HIVepidemicandtheneedforcontinuedresearchintoHIV pathologyandtreatment.
HIVbelongstothefamily Retroviridae,agroupofRNA virusescharacterizedbytheiruseofreversetranscriptasetomake complementaryDNA(cDNA)copiesoftheirgenomethatarethen integratedintothehostcellgenome(Krebsetal.,2002).HIV typicallyrefersspecificallytoHIV-1–thevirusthatmakesupthe vastmajorityofglobalHIVinfectionsandover99.9%ofHIV infectionsintheUnitedStates–asopposedtoHIV-2,amuchrarer
virus(Peruskietal.,2020).MatureHIV-1viralparticleshavean exteriorlipidbilayerderivedfromthehostcellmembranethat containsviralglycoproteins(Figure1).Interiortothemembraneis thematrix,aproteinaceousshellthatenclosestheviralcontents.At thecenterofthevirusistheviralcoreenclosedbyaconical capsid,whichcontainstheviralRNAalongwithnucleocapsid proteins,integrase,andreversetranscriptase.TheHIV-1genomeis approximately10kilobaseslong(Figure2).Atthestartandendof thegenomearethe5’and3’longterminalrepeats(LTRs),which eachcontaina5’anda3’untranslatedregion(UTR)aswellasa seriesofrepeatedbasepairs(Krebsetal.,2002).The5’LTRacts asthecanonicalpromoterfortheHIVgenome,bindingbothhost celltranscriptionalproteinsaswellasviralregulatoryproteinsto initiateandmodulatetranscription;the3’LTRprimarilyregulates polyadenylationoftranscripts.Inadditiontotheseregulatory sequences,theHIVgenomecontainstheGroup-specificantigen (Gag)region,whichencodescapsidproteinssuchastheprecursor p55myristoylatedproteinanditsderivatives;thepolymerase(pol) region,whichencodestheviralenzymesreversetranscriptase, integrase,andprotease;theenvelope(env)region,whichencodes theviralglycoproteinsgp120andgp41;aswellasvariousother regionsencodingforregulatoryproteins(LosAlamosNational Laboratories,n.d.).
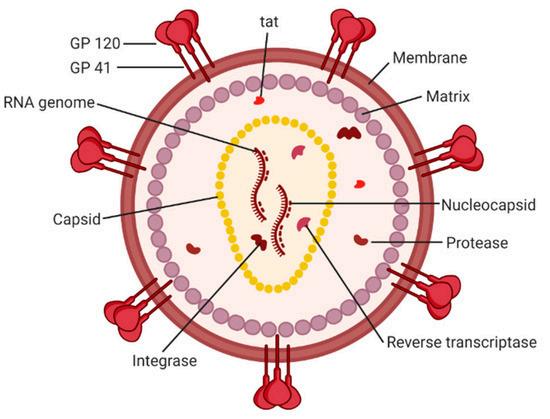
Figure1:DiagramofmatureHIV-1viralparticles(Rossietal., 2021).
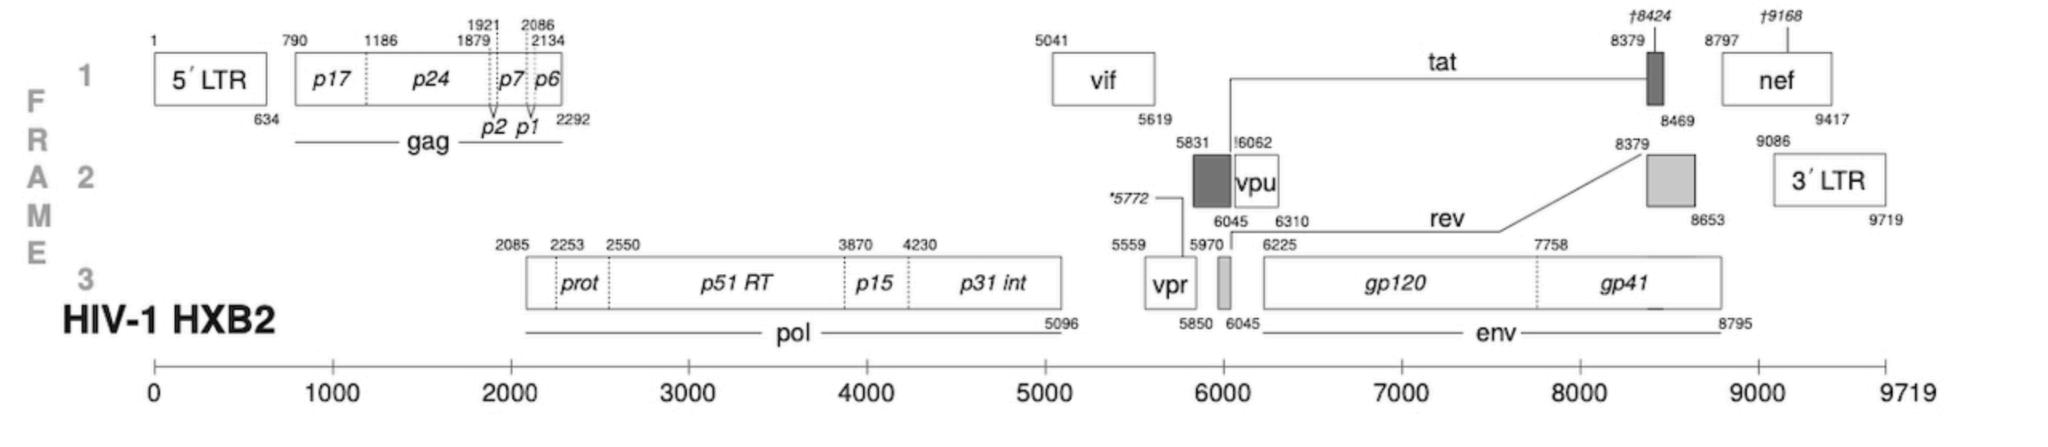
Figure2:ConfigurationoftheHIV-1genomebasedonthe subtypeBreferencesequenceHXB2.TatandRevexonsare shownshadedingray,whileotherregionsandgeneproductsare showninwhite(LosAlamosNationalLaboratories,n.d.).
AIDSwasfirstidentifiedin1981throughtheriseof Kaposi’ssarcomaandpneumocystiscariniipneumonia—bothrare conditionsassociatedwithimmunosuppression—inyoung,
otherwisehealthymenlivinginUSmetropolitanareas(DavidJ. SencerCDCMuseum,2024).In1983,HIVwasidentifiedasthe causativepathogenbehindAIDS(Schmid,2018).Initially, HIV/AIDSwasanuntreatableterminalcondition;ofthe593cases ofHIVreportedtotheCentersforDiseaseControlandPrevention (CDC)betweenJune1981andSeptember1982,41%ofthose casesresultedindeathbylateSeptember1982(Centersfor DiseaseControlandPrevention,1982).However,in1987,the reversetranscriptaseinhibitorazidothymidine(AZT) was approvedbytheFoodandDrugAdministration(FDA)asthefirst antiretroviraldrugtotreatHIV(NationalInstituteofAllergyand InfectiousDiseases,2025).In1996,proteaseinhibitorswere approvedbytheFDAasanewclassofantiretroviraldrugswhich, incombinationwithreversetranscriptaseinhibitors,candurably suppressHIVindefinitelyprovidedtreatmentisnotinterrupted (NationalInstituteofAllergyandInfectiousDiseases,n.d.).New classesofantiretroviraldrugsdevelopedsince1996,including non-nucleosidereversetranscriptaseinhibitors,entryandfusion inhibitors,andintegraseinhibitorshaveimprovedtheeffectiveness ofantiretroviraltherapy(ART).TheseHIVtreatmentshave dramaticallyimprovedthelifeexpectancyofpeoplelivingwith HIV;whereasinthe1980s,mostpeoplewithHIVdiedofAIDS withinafewyears,ARThasextendedthelifeexpectancyof peoplewithHIVtonear-normalprovidedthattheybeginART withsufficientlyhighwhitebloodcellcounts(Trickeyetal., 2023).ThisshiftfromHIVasanacutediseasetoHIVasachronic conditionhascreatednovelchallengesintreatingHIV.
OnesuchchallengeinmanagingchronicHIVissystemic inflammation;HIVinfectionisassociatedwithavarietyofchronic non-communicableinflammatorydiseases,includingheartdisease andneurocognitivedisorders.HIVinfectioniscorrelatedwitha 1.5totwofoldincreaseinacutemyocardialinfarctionrateswhen
adjustedforcommonriskfactors(Triantetal.,2007).Furthermore, peoplewithHIVhaveanelevatedriskofdevelopingacute coronarysyndrome(ACS)—whichincludesunstableanginaand myocardialinfarctions—againwithinayearafteraninitialACS episode(Boccaraetal.,2010).Increasedriskofmyocardial infarctioniscorrelatedwithlowerCD4+Tcellcountsandhigher viralRNAlevels,suggestingalteredimmuneresponsesmay contributetotheriskofadversecardiovasculareventsinpeople livingwithHIV(Drozdetal.,2018).HIVisalsoassociatedwith neurocognitivedysfunction(Rosenthal&Tyor,2019).AsHIV becomesamorechronicconditionandasthepopulationofpeople withHIVages,therehasbeenanincreaseinHIV-associated neurocognitivedeficits(HAND).Estimatesforthepercentageof peoplelivingwithHIVwithHANDrangefrom33%to52% dependingonthestudy(Rosenthal&Tyor,2019).HIVisbelieved topenetratethecentralnervoussystemearlyininfection,andsince ARThaspoorpenetrationoftheCNSduetotheblood-brain barrier,neuroinflammationcontinuesevenwithundetectableviral RNAlevels.HANDisassociatedwithelevatedmarkersof monocyteactivation,whichsuggestsalinkbetweeninflammatory responsesandneurocognitivedisordersinHIV(Abutaleb& Feinstein,n.d.;Burdoetal.,2011).Ultimately,theconfluenceof bothcardiovascularandneurologicalinflammatoryconditionsin peoplelivingwithHIVsuggeststhepresenceofunderlying inflammatoryresponsesinchronicHIVinfection.
Onepossiblemechanismdrivingthischronicinflammation istheaccumulationofdefectiveproviraltranscripts;multiple factorscontributetothegenerationofalargepoolofdefective provirusesinpeoplelivingwithHIV,thetranscriptionofwhichis suspectedtocontributetochronicinflammationthroughmultiple distinctmechanisms(Kilroyetal.,2024).Adefectiveprovirusisa pieceofviralDNAintegratedintothehostcellgenomethatis
unabletoproduceafunctionalvirus.Defectiveprovirusesare generatedthroughmultiplemechanisms,includingerroneous reversetranscription,cellularrestrictionfactors,andDNAdamage responses.Reversetranscriptaselacksproofreadingcapabilities andispronetotemplateswitching,whichcanleadto hypermutationandinternaldeletionsintheHIVgenomethat renderitdefective.Furthermore,restingCD4+Tcells, monocyte-derivedmacrophages(MDMs),andmacrophages derivedfrominducedpluripotentstemcellsallcontainrestriction factorsthatmaylimitreversetranscription.Forexample,the restrictionfactorSAMHD1reducesthenucleotideconcentrationin cells,possiblycontributingtodefectiveproviruses.Additionally, DNAdamagerepairinvolvedinDNAintegrationisanother error-proneprocessthatcouldcontributetothedefectivereservoir. Cellswithdefectiveprovirusesmayescapeselectiveimmune pressures,allowingfortheexpansionofthisreservoirovertime. Thus,thereareseveralmechanismsthatcontributetothe generationofdefectiveproviraltranscripts,includingbutnot limitedtoerroneousreversetranscription,thepresenceofcellular restrictionfactors,andDNAdamageresponsepathways.
ThemRNAsgeneratedfromdefectiveprovirusesare hypothesizedtocontributetochronicinflammationinpeople livingwithHIV.PeoplelivingwithHIVundergoingARTcontinue tohaveelevatedlevelsofproinflammatorycytokinesthatsuggest persistentinflammationonthecellularlevel,whichisconsistent withtheacceleratedaging,increasedriskofadversecardiac events,andneurologicaldisordersassociatedwithlong-termHIV infection(Kilroyetal.,2024).Therearemultiplepotential explanationsforthisphenomenon.First,defectiveviralRNAsmay serveasintracellularpathogenassociatedmolecularpatterns (PAMPs)thatactivatepathogenrecognitionreceptors(PRRs), whichdriveinflammation.Second,defectiveprovirusesmaylack
mechanismstoevadetheinnateimmunesysteminmyeloidcells duetoalteredsplicingpatterns.Forexample,unsplicedRNAsthat containintronscantriggerinnateimmuneresponsesviaactivation ofmitochondrialantiviralsensingprotein-mediatedinterferon responsesinmacrophagesandthroughcytosolicsensing mechanismsinmicroglia(Akiyamaetal.,2021;Ramaswamyet al.,2025).Third,humanendogenousretroviruses(HERVs)are knowntocompriseroughly8%ofthehumangenome,butare typicallysilencedthroughepigeneticfactorsorothermechanisms. However,HIVmayupregulatetranscriptionofHERVs,providing anothersetofPAMPsthatcouldcontributetoinflammation. Regardlessoftheexactmechanism,defectiveproviraltranscripts likelycontributetocellular-levelchronicinflammatoryresponses inpeoplelivingwithHIV.
Kuniholmetal.identifieddefectiveHIV-1transcripts originatingfromanintragenictranscriptionalelement(2021). CanonicalHIV-1transcripts—ortranscriptsoriginatingfromthe5’ LTR—alwayscontaintheuniversalsplicedonor(U5)region. Kuniholmetal.identifiedtranscriptsinCD4+TcellsandMDMs thatcontaintheenveloperegionoftheHIV-1genomebutlackthe U5region.Thesetranscriptscontainonlyroughlythelatterhalfof theHIVgenome.Thisfindingimpliestheexistenceofa non-canonicalintragenictranscriptionalelementthatservesasan alternativepromoterforHIV-1.Notably,theseU5deficient transcriptswerealsoidentifiedinasubsetofpeoplewithHIVon ART,suggestingthattheymaybeclinicallyrelevant.Kuniholmet al.thenidentifiedaspecificsubsectionoftheenveloperegionof theHIVgenomethatcouldexplainthesedefectivetranscripts.This envelope-regionpromoterispostulatedtocontributetothe accumulationofdefectiveproviraltranscripts,whichinturnmay contributetochronicinflammatoryresponsesinpeoplelivingwith HIV.
Whetherthisenvelope-regionintragenictranscriptional element(ITE)alsobehavesasanenhancerintheHIVgenomeis anongoingquestionthathasimplicationsforunderstandingthe mechanismsdrivingHIVviralreplicationandchronic inflammation.LuciferasereporterassaysinvolvingtheITEwere usedtoevaluatethepotentialenhanceractivityofthisenvelope regionsequenceandtomorebroadlycharacterizeits transcriptionalactivity.Theresultsshowthat,comparedtoother regionsoftheHIVgenome,theenvelope-regionITEupregulates transcriptionofluciferasewhenclonedinfrontofaminimal promoterandluciferasereportergene.IftheITEregionbehaved strictlyasapromoter,onewouldexpectluciferaseexpressionto decreasecomparedtocontrolsequencesduetointerference betweenpromoters.Thus,theupregulationofluciferaseexpression whentheITEisclonedinfrontofaminimalpromotersuggests thatthisregionbehavesasanenhancer.Thisfindingfurther illuminatesthemechanismsdrivingtheaccumulationofdefective proviraltranscriptsinpeoplelivingwithHIV,withthegoalof ultimatelyaddressingHIV-associatedchronicinflammation.
Methods
Sequences
Theenvelope-regionITEwasdefinedasTile14in Kuniholmetal.’sidentificationoftranscriptionallyactiveHIV-1 sequencesinNL43(2021).Asequencefromthepolyprotein(pol) regioncorrespondingtoTile5inthisdatasetwaschosenasa controlsequencetotheITEbecauseofitslackoftranscriptional activity.
PlasmidGeneration
ModifiedplasmidsweregeneratedusingNEBuilderQ5 High-FidelityDNAPolymerasePCRamplificationofbothNL43 backbonesequencesandaminimalpromoterdrivenfirefly luciferasevector.Theluciferasevectorcontainedaminimal promoterinfrontofaluc2luciferasereporter,aswellasan ampicillinresistancegeneandarestrictionsitebeforetheminimal promoter(Figure3).PCRamplificationoftheITE,polsequence, andtheminimalpromotervectorwasconductedaccordingtoQ5 High-FidelityDNAPolymerasePCRProtocol(NewEngland Biolabs,n.d.).Forpolsequenceamplification,Region5Forward withSacIRestrictionEnzymeandRegion5ReversewithXhoI RestrictionEnzymeprimersasdefinedbyKuniholmetal.were utilized(2021).Likewise,forITEamplification,Region14 ForwardwithSacIRestrictionEnzymeandRegion14Reverse withXhoIrestrictionenzymewasused.
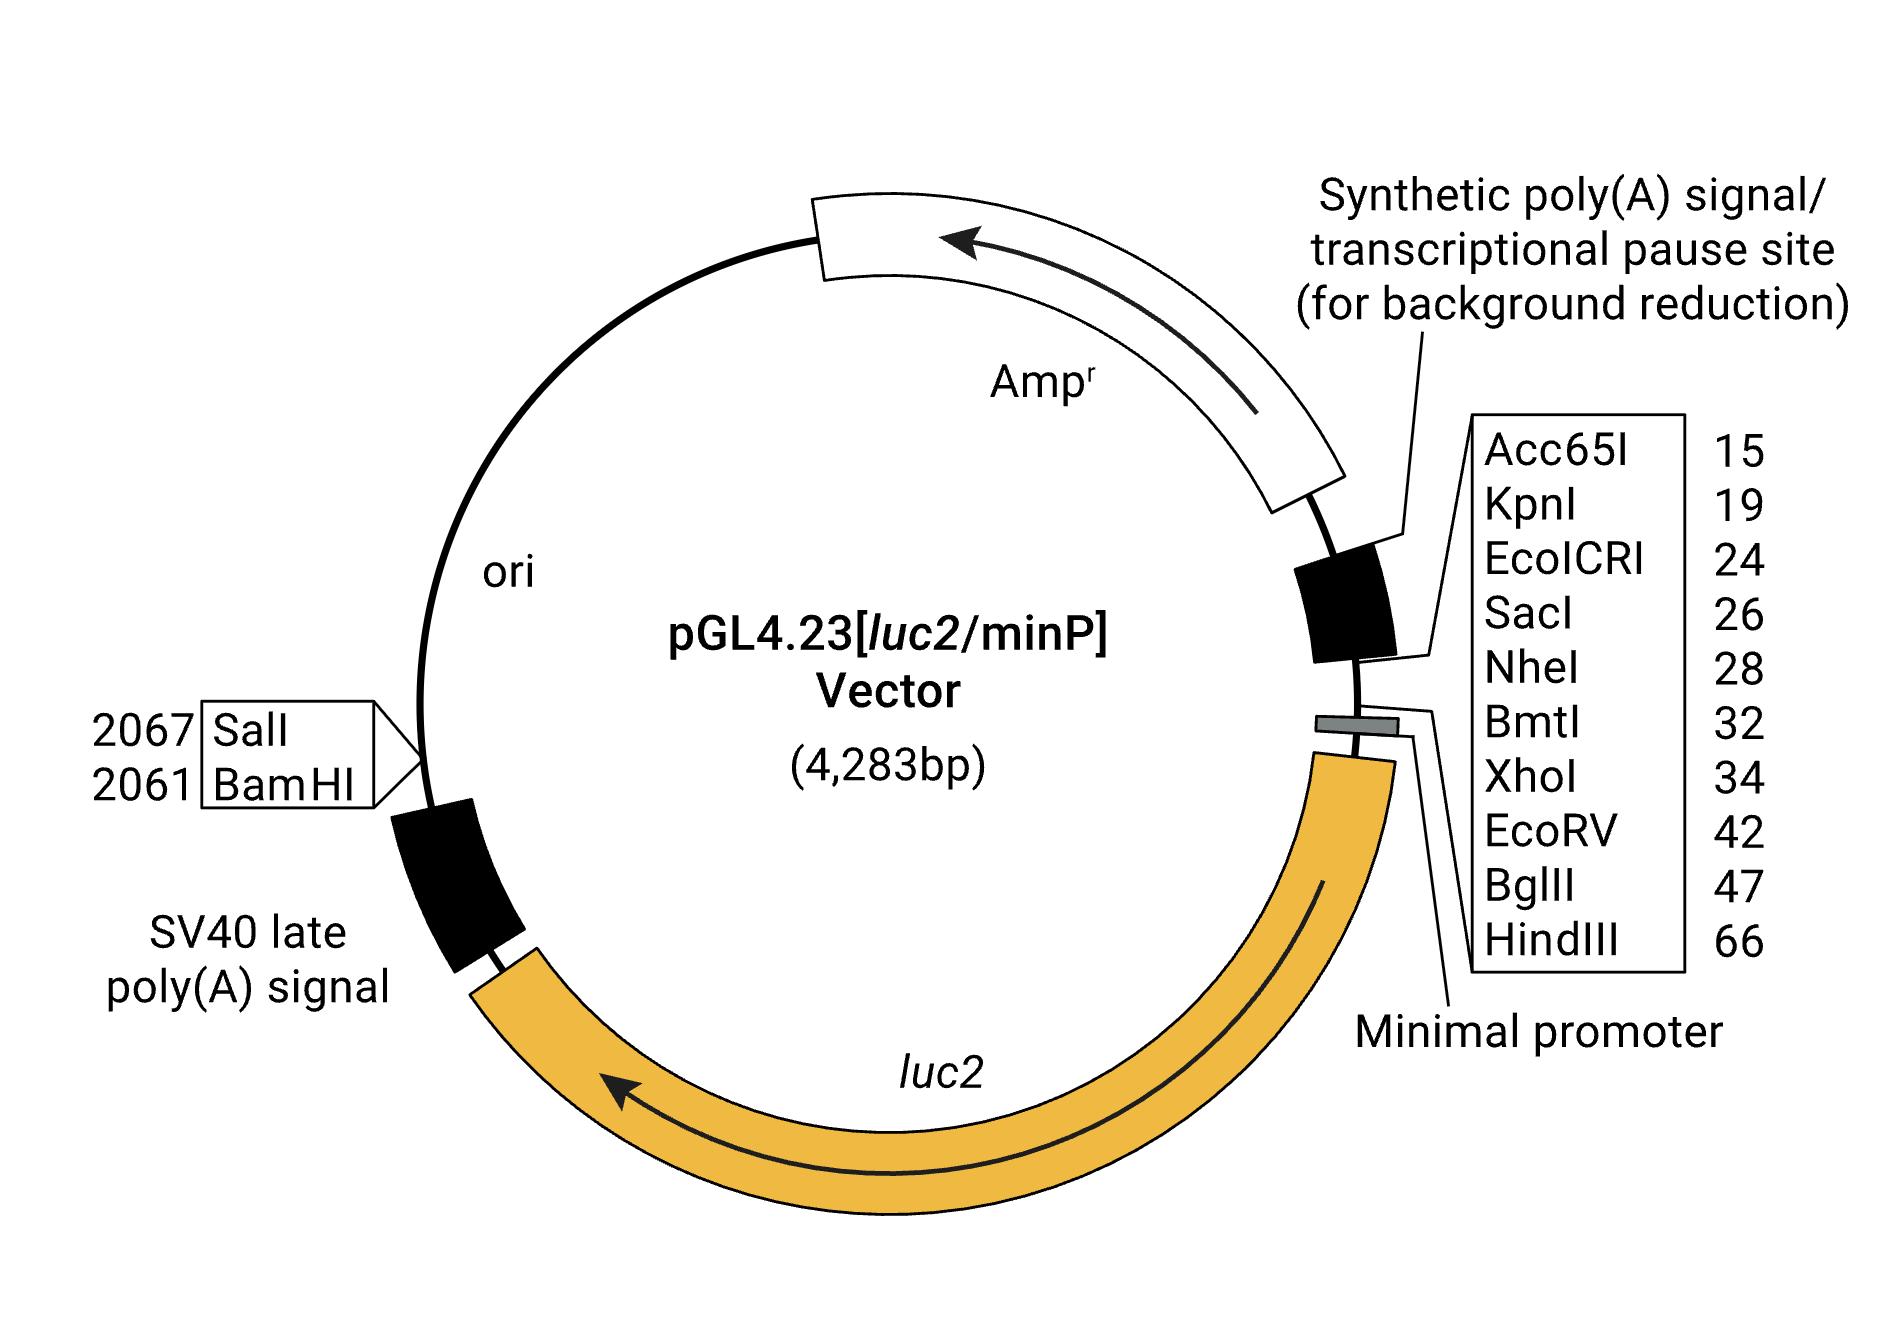
Figure3:Theuneditedluc2minimalpromoterdrivenfirefly luciferasevector.NotetheSacIandXhoIrestrictionsitesadjacent totheminimalpromoter.
Amplificationwasconfirmedusinggelelectrophoresis. Sampleswererunonagelcontaining0.8%agarand1μLofgel redper10mlofagarsolutionat85Vfor40minutes.QuickLoad Purple1kbLadderwasusedtoconfirmthatthelengthofthe amplifiedregionswasconsistentwithexpectedlengths.Plasmids werethenassembledusingarestrictionenzymedoubledigestand T4ligation.TherestrictionenzymesSacI-HSandXhoIwereused accordingtotheNEBclonerRestrictionEnzymeDoubleDigestion protocol(n.d.).Therestrictionsiteslocatednexttotheminimal promoterontheminimalpromotervector,andappropriate restrictionsitesoneithersideofthepolregionandITEinserts, allowedforeffectiveconstructionofthisplasmid(Figure4). LigationwasperformedusingNewEnglandBiolabs’Ligation ProtocolwithT4DNALigase(n.d.).
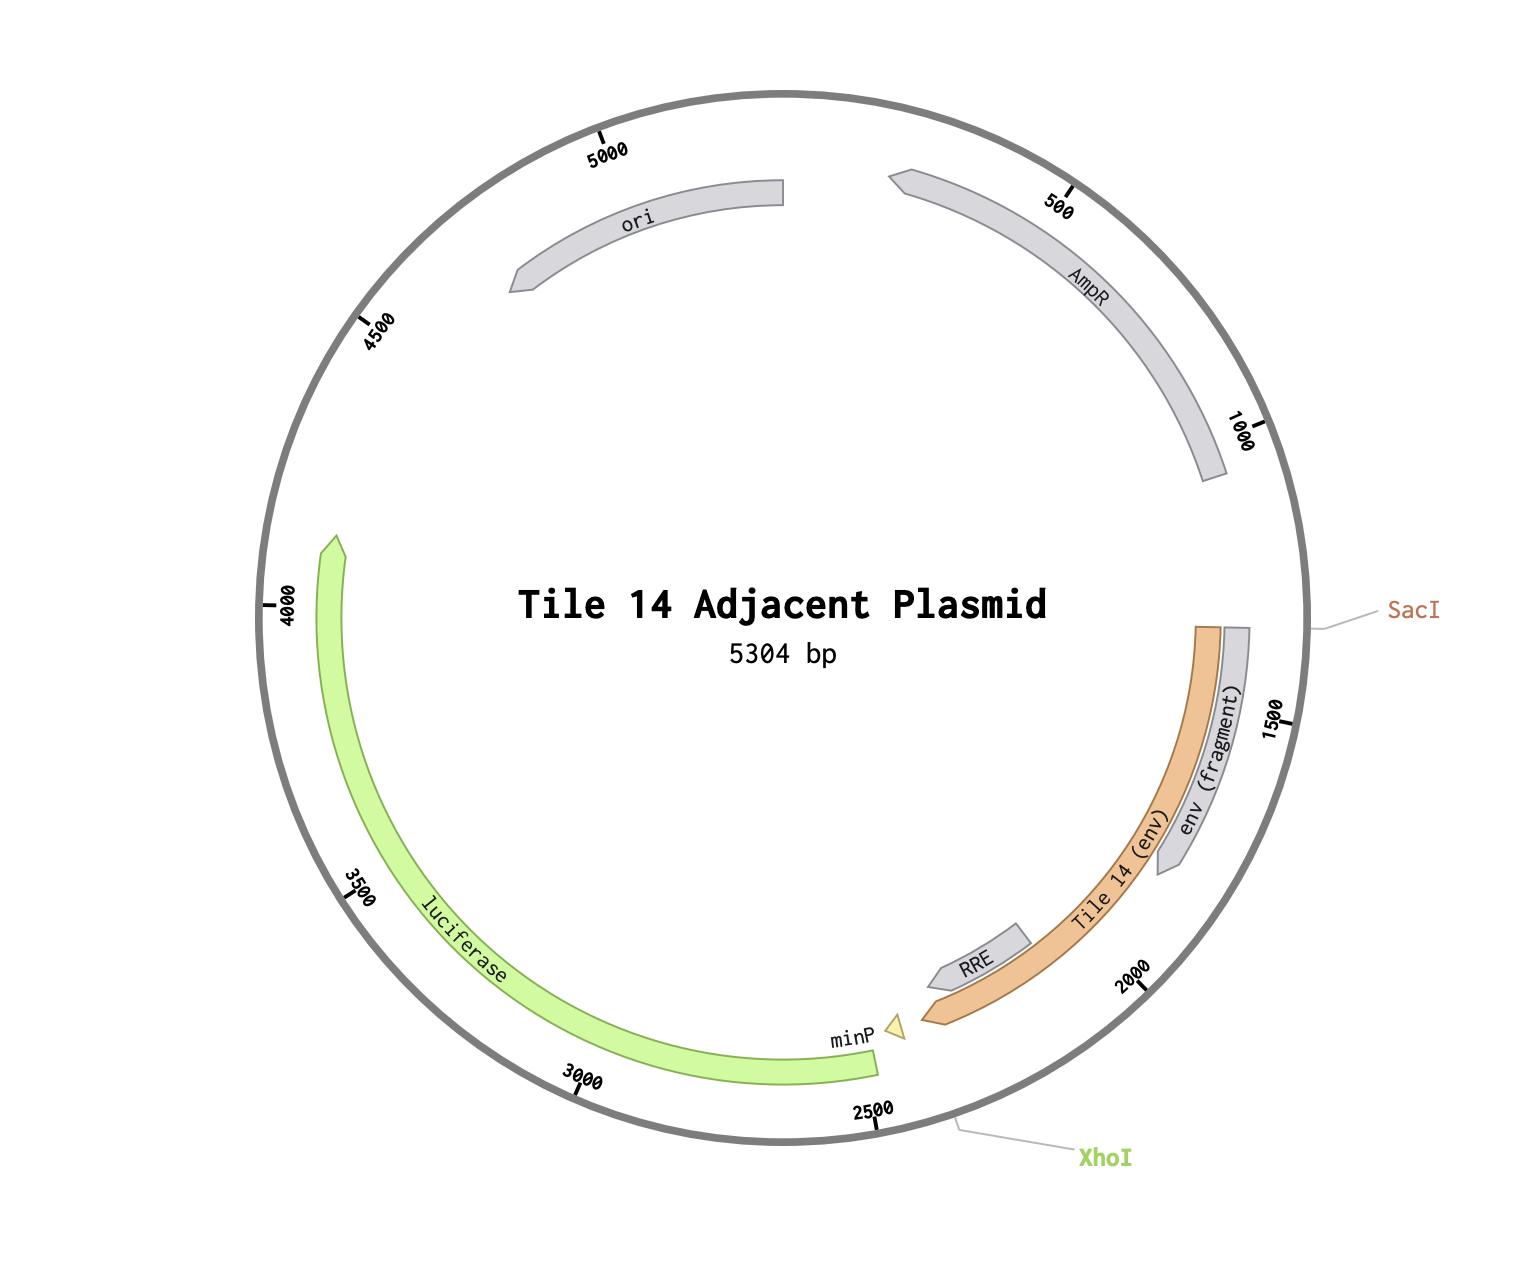
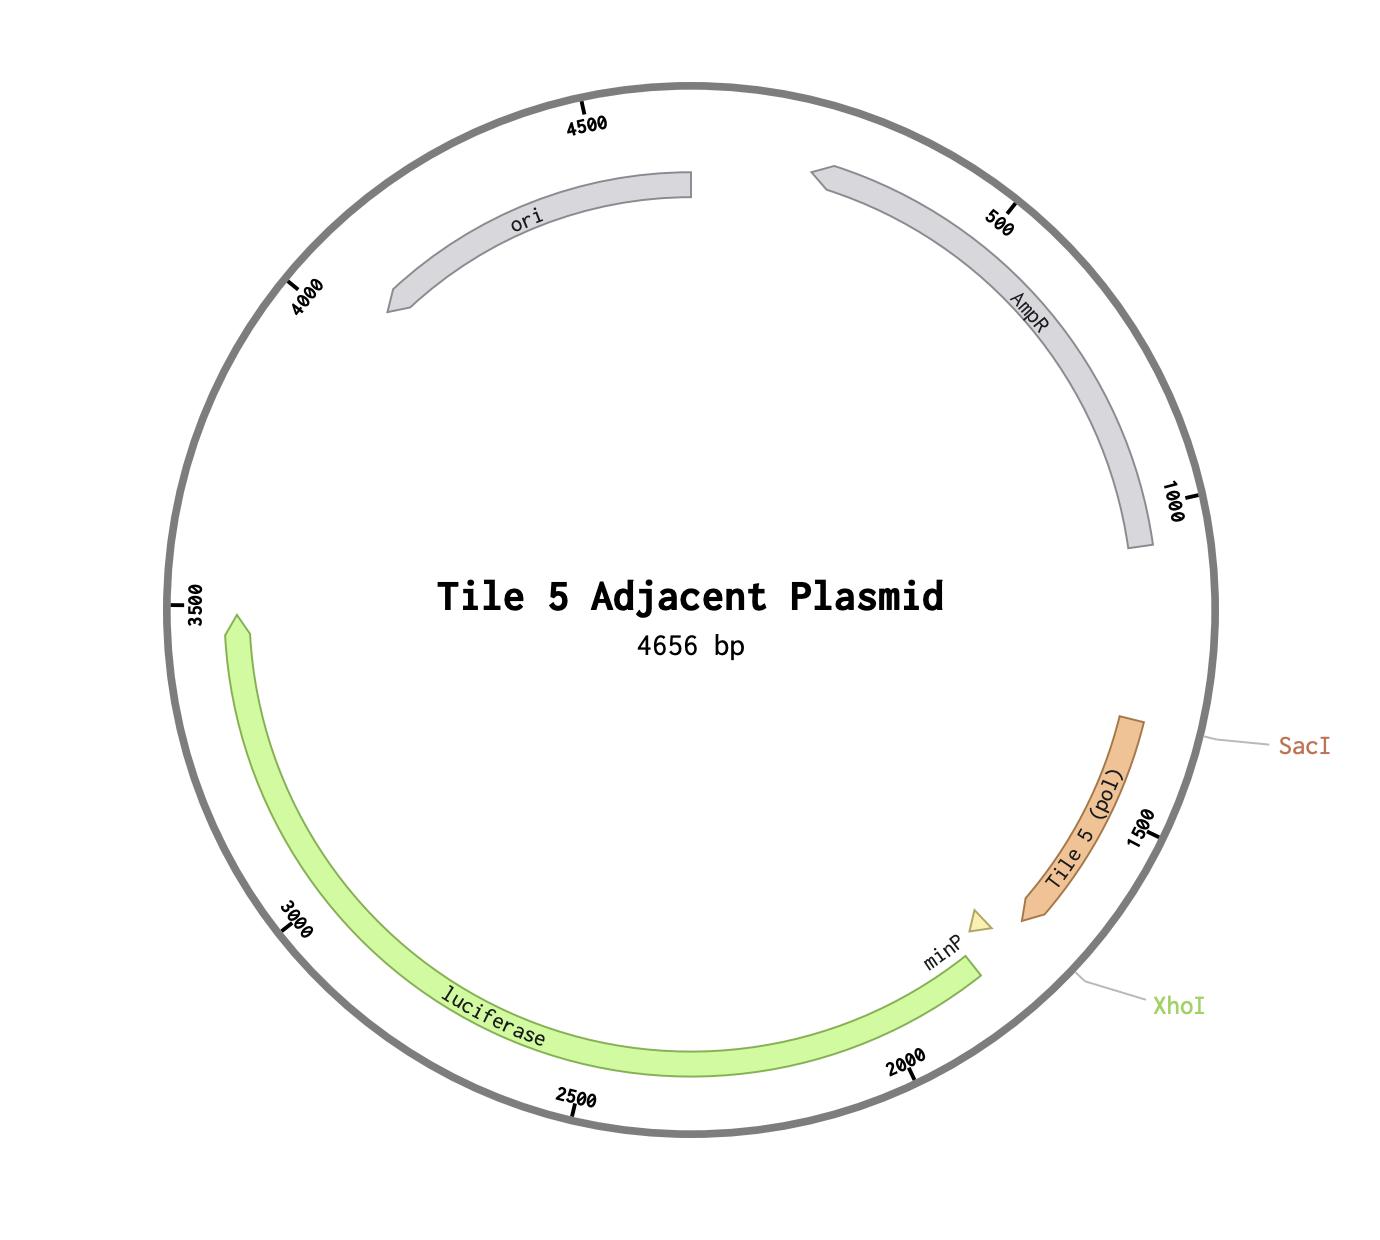
Figure4:Configurationofthepromoterdrivenfireflyluciferase vectorswithHIVenvelope-regionITE(left)andpolregion(right) inserts.minPreferstotheminimalpromoter.
PlasmidSelection
Modifiedplasmidswereselectedthroughtransformation into E. coli TOP10s.Bacterialcellswerethawedonicebefore transformation.Asmallamount(1uL)ofDNAwasthenaddedto bacterialcells.Thecellswereelectroporatedandresuspendedin SuperOptimalbrothwithCataboliteexpression(SOC).The outgrowthwasincubatedinashakerat~225rpmand37°Cfor1 hourandthenspreadontoLBagarplatescontainingcarbenicillin andincubatedat37°Cfor24hours.Colonieswerethenselected andincubatedinLBbrothcontainingcarbenicillininashakerat 37°Cfor24hours.Sincetheplasmidscontainedampicillin resistancegenes,anycoloniesthatgrewincarbenicillin-containing mediahadbeeneffectivelytransformed.Plasmidswerethen isolatedfromcellsusinganinvitrogenPureLinkQuickPlasmid Miniprepkit.Thepropersequencingandorientationofthe plasmidswasconfirmedusingPlasmidsource.
TissueCulture
ThisexperimentutilizedHEK293Ts.Stockcellswere thawedandwashedtwicewithphosphatebufferedsaline(PBS). CellswerethenresuspendedinDMEM(containing10%fetal bovineserum,1%penicillin-streptomycin,and1%L-glutamine)at aconcentrationof1x10^5cellspermilliliterandtransferredtoa T75flask.Cellswereincubatedat37°Cand5%carbondioxide. Cellsweresplit1:10onalternatingdaysbyremovingoldmedia, washingcellswithPBS,detachingcellsfromtheflaskwith 0.025%trypsinandethylenediaminetetraacetic acid,andseeding cellsinanewT75.
Transfection
HEK293Tsonapproximatelypassage4wereseededina white-walled96-wellplate.Cellswereseededin100μLof DMEMmediaperwellataconcentrationof2x10^5cellsper milliliter.Cellswerethenincubatedat37°Cand5%carbon dioxidefor20hoursuntiltheyreachedapproximately70% confluency.HEK293TsweretransfectedusingLipofectamine3000. ReagentsweredilutedwithOptiMEMandaddedtosamples accordingtoanadaptedversionofLipofectamine3000Reagent Protocol(invitrogen,2016).Conditionsforthistransfection includedpolregion-luciferaseandrenilla,ITE-luciferaseand renilla,polregion-luciferaseonly,ITE-luciferaseonly,minimal promotor-luciferaseandrenilla,minimalpromotor-luciferaseonly, renillaonly,andcellsonly.VaryingamountsofplasmidDNAwas addedtoaccountforthecopynumberofeachplasmid.90ngof DNAwasaddedtoeachITEconditionsincetheITE-luciferase plasmidwasthelargest.79ngofDNAwasaddedtoeachpol region-luciferasecondition,and72.6ngofluciferasevectorDNA withnoinsertwasaddedtoeachminimalpromotor-luciferase condition.Thesequantitieswerecalculatedtonormalizetothesize ofeachplasmidandthecorrespondingrateoftranscription.10ng ofrenillaluciferasewasaddedtoeachoftherenillapositive conditions.TheamountsofOptiMEM,Lipofectamine3000,and P3000werethenscaledtoaccountforthesevaryingamountsof DNA.(Forthecellsonlyandrenillaonlycontrolconditions,these quantitieswerecalculatedasifthewellscontained100ngof DNA.)AftertheadditionofLipofectamine3000,thesolutions wereincubatedfor15minutesandthenaddedtoplated HEK293Ts,withthreewellspercondition.
TheDual-GloLuciferaseAssaySystemwasutilizedtoread outluciferasereporters.Theprotocolfromthemanufacturerfor
thisexperimentwasmodifiedslightly;50μLofmediawas removedfromthewellsandthen50μLofDual-GloReagentwas addedtothewells.Likewise,50μLofDual-GloStop&Glo reagentwasaddedafterreadingfireflyluciferase(Promega,2025). Thismodificationwasmadetoconservereagentsandlikelyhadno effectontheefficacyoftheexperiment.
Results
Inordertodeterminethecis-regulatoryactivityofthe enveloperegion,wegeneratedplasmidswiththeITEclonedin frontofaminimalpromoterandluciferasereportergene.Higher luciferaseluminescencecorrespondstohigherlevelsofluciferase geneexpression,whichindicatesincreasedtranscriptionalactivity. Thisexperimentusedplasmidconstructsthatcontainedeitherthe polregioncontrolsequenceortheITEsequenceclonedinfrontof aminimalpromoterandfireflyluciferasereporter.Because adjacentpromoterstypicallyinterferewitheachother,increased luciferasereporterreadoutintheITE-luciferaseplasmidsample comparedtothepolregion-luciferasecontrolsamplewould suggestthattheITEsequencebehavesasanenhancerratherthan solelyasapromoter.
Sincerelativeluminescencemustbestandardizedto backgroundlevelsofexpression,Renillaluciferaseconstructswere usedinsomeexperimentalconditions;thisenabledthe luminescenceoffireflyluciferasetobestandardizedtoRenilla luciferasebackground.
Therelativefireflyluciferaseluminescenceofthe ITE-luciferase+renillaconditionwasgreaterthanthe luminescenceofthepolregion-luciferase+renillaconditionforall samples(Table1).Thepolregion-luciferaseonlyand ITE-luciferaseonlyconditionswereusedtoconfirmthatthe additionofRenillaluciferasedidnotinhibittheexpressionof
fireflyluciferase;thehigherluminescenceintheRenillaconditions suggeststheRenillaluciferaseconstructdidnotinterferewiththe fireflyluciferaseconstruct(Table1).Additionally,firefly luciferasereadoutforboththepolregion-luciferase+renillaand ITE-luciferase+renillaconditionswassignificantlylowerthanthe minimalpromoter-luciferase+Renillaconditionreadout(Table1). Thissuggeststhatcloninganysequenceinfrontoftheminimal promoter-luciferaseconstructdecreasesluciferaseexpression, regardlessofthetranscriptionalactivityofthatsequence. However,thiseffectcanbedisregardedbecauseitislikelytobe theidenticalforboththeITE-luciferaseandpolregion-luciferase conditions.
Table1:Fireflyluciferasereporterreadout.Relativeluminescence units(RLU)forfireflyluciferaseineachexperimentalcondition.
Condition
Renillaluciferasereadoutprovidesamechanismwith whichtostandardizefireflyluciferasereadoutforconditions
containingbothfireflyluciferaseandRenillaluciferase.Whilethe Renillaluciferasereadoutfortheminimalpromoter-luciferase+ Renillaconditionwasabnormallyhigh,theRenillaluciferase readoutwascomparabletothefireflyluciferasereadoutforthis condition(Table2).Furthermore,asexpected,theRenilla luciferasereadoutwassimilaracrossthepolregion-luciferase+ renillaandITE-luciferase+renillaconditions.Thissuggeststhat theRenillaluciferasereadoutisreliableandcanbeusedto standardizefireluciferaseexpression.
Table2:Renillaluciferasereporterreadout.RLUforRenilla luciferaseineachexperimentalcondition.
Condition
Thefoldchangeinluminescencebetweenthefirefly luciferasereadoutandtheRenillaluciferasereadoutwascalculated forthepolregion-luciferase+renilla,ITE-luciferase+renilla,and minimalpromoter-luciferase+renillaconditions(Table3).Firefly luciferasereadoutwasdividedbyRenillaluciferasereadoutfor
eachsample,andthesequantitieswereaveragedacrosstechnical replicatesforeachexperimentalcondition.Foldchange calculationsstandardizetheluminescenceofeachwellandenable furtherdataanalysis.Theaveragefoldchangeinluminescencewas greaterfortheITE-luciferase+renillaconditioncomparedtothe polregion-luciferase+renillaandminimalpromoter+renilla conditions(Table3).ThissuggeststhattheITEincreased luciferaseexpressioncomparedtoboththepolregion-luciferase controlconditionandtheminimalpromoter-luciferasecontrol condition.Furthermore,asexpected,theaveragefoldchangein luminescencebetweenfireflyluciferaseandRenillaluciferasewas similarforthepolregion-luciferase+renillaandminimal promoter-luciferase+renillaconditions(M=1.17andM=1.22, respectively).Thissuggeststhatthepolregionhadnoadditional transcriptionalactivitycomparedtothepromoterandfurther confirmsthereliabilityoftheassay.
Table3:Standardizedrelativeluminescenceunitsoffirefly luciferaserelativetoRenillaluciferase.
Minimalpromoter-luciferase+
Thefoldchangeinluminescencebetweenfireflyand Renillaluciferasewasplottedforboththepolregion-luciferase+ renillaconditionandtheITE-luciferase+renillacondition(Figure 5).Analysisshowedthattherewasasignificantdifferencein
relativeluminescencebetweenthepolregionandtheITE(paired t-test,p<0.001).
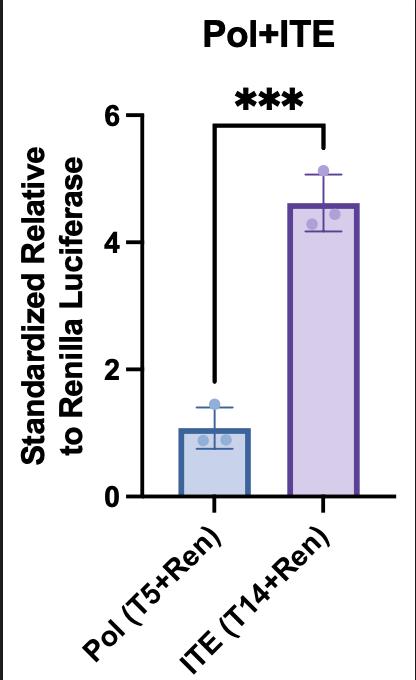
Figure5:Foldchangeinpolregionluminescence(blue)andITE luminescence(purple)relativetoRenillaluciferase.
Thesignificantincreaseinstandardizedfireflyluciferase expressionintheITE-luciferase+renillaconditioncomparedto thepolregion-luciferase+renillaconditionindicatesthattheITE upregulatestranscriptionwhenclonedinfrontofaminimal
promoter.Sinceadjacentpromoterstypicallyinterferewitheach other,causingeitheradownregulationofexpressionornochange inexpression,thisfindingsuggeststhattheITEbehavesasan enhancer.
Discussion
TheseresultsillustratethatcloningtheITEinfrontofa minimalpromoterandluciferasereportergeneincreasedluciferase geneexpressionrelativetopol-regioncontrolsequences.The averagefoldchangeinfireflyluciferaseluminescencerelativeto RenillaluciferaseoftheITEsampleswassignificantlygreaterthan theaveragefoldchangeofthecontrolsamples(Table3andFigure 5,p<0.001).ThesefindingsillustratethattheITEhas transcriptionalactivitywhenclonedinfrontofaminimal promoter,whichfurthercorroboratespreviousfindingsthatthis regionistranscriptionallyactive(Kuniholmetal.2021).More specifically,theseresultssuggestthattheITEactsasa cis-regulatoryelementintheHIVgenome.IftheITEwassolelya promoter,theresultswouldlikelyhaveshowneithernochangeor adecreaseinluciferaseexpressioncomparedtocontrolsequences duetointerferencewiththeminimalpromoter.Theincreasein luciferaseexpressionintheITEplasmidscomparedtocontrol plasmidsthereforesuggeststhattheITEbehavesasa cis-regulatoryelement.
Asthiswasafairlypreliminarystudy,moreresearchis neededtocorroboratethesefindingsandfurthercharacterizethe intragenictranscriptionalactivityoftheITE.Alimitationofthis studyisthatitdoesnotexaminethetranscriptionalactivityofthe ITEinHIV-infectedcells.Thus,anotherfutureexperimentisa chromatinimmunoprecipitationassay(ChIP)ofHIV-infected CD4+TcellsinconjunctionwithaddPCRanalysisofboth canonicalandnoncanonicalHIVtranscriptsinthesecells.This
experimentwouldrelatemethylationmarksontheHIVgenome withviraltranscriptsisolatedfrominfectedcells.Correlation betweenadecreasemethylationmarksintheenveloperegionand anincreaseinU5deficientproviraltranscriptswouldfurther suggestthattheITEactsasapromoterregioninlymphoidcells. Furthermore,acorrelationbetweenadecreaseinenvelope-region methylationandanincreaseinnormalproviraltranscriptscould suggestthattheITEupregulatesnormalLTR-driventranscription throughenhanceractivity.Anotherfutureexperimentinvolves creatingplasmidconstructswheretheITEandpolregioncontrol sequenceareclonedoppositetheminimalpromoterandrepeating theluciferasereporterassayconductedinthisstudy(Figure6). Theabilitytoupregulateordownregulategeneexpressionevenfar fromthetargetgeneitselfispartoftheclassicdefinitionofan enhancer.Thus,anincreaseinluciferaseexpressioninITEplasmid samplescomparedtocontrolsampleswhentheseregionsare locatedoppositetheminimalpromoterwouldfurthersupportthe hypothesisthattheITEactsasacis-regulatoryelement. Additionally,iftheITEregulatorysequenceisindeedanenhancer, itshouldalsobeabletoactdownstreamofatargetgeneto upregulatetranscription.Thus,anotherpotentialexperimentto furthercharacterizetheregulatoryactivityoftheITEisarepeatof theluciferasereporterassaybutwiththeITEandpolregioncloned downstreamofaminimalpromoter.
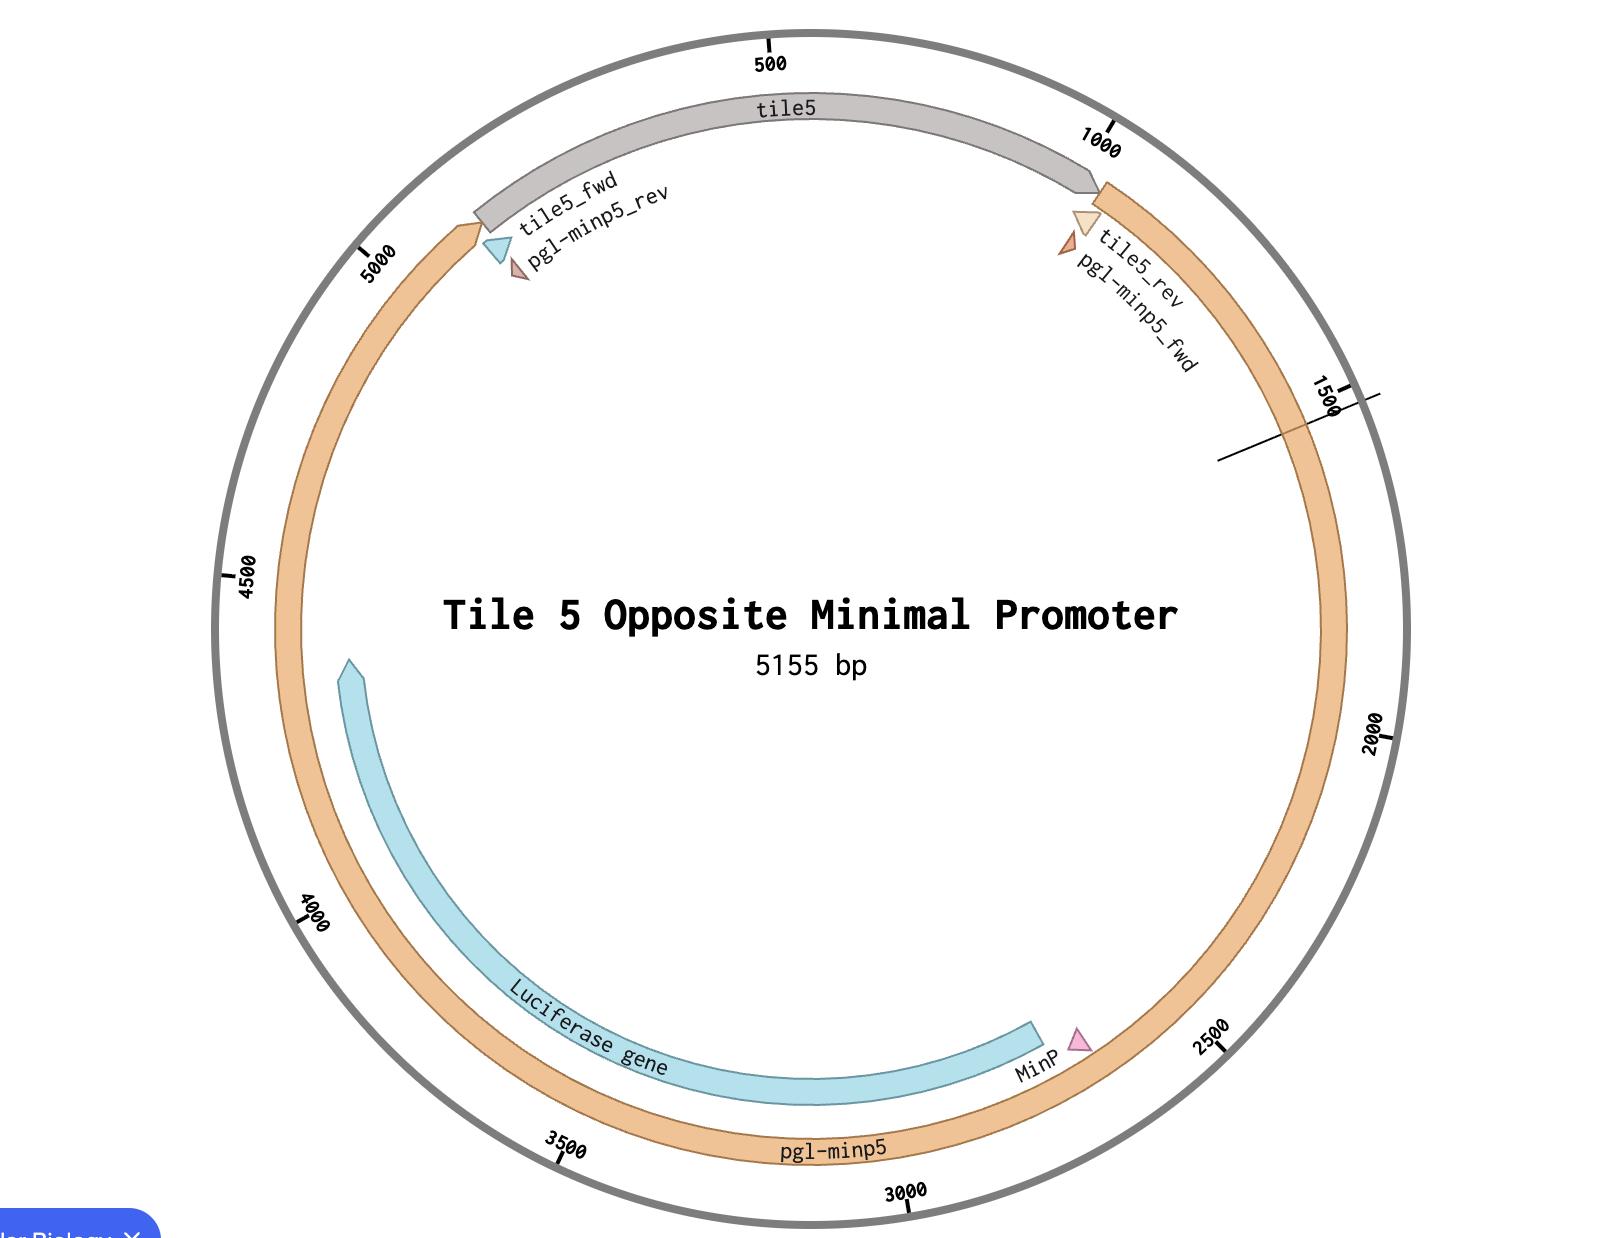
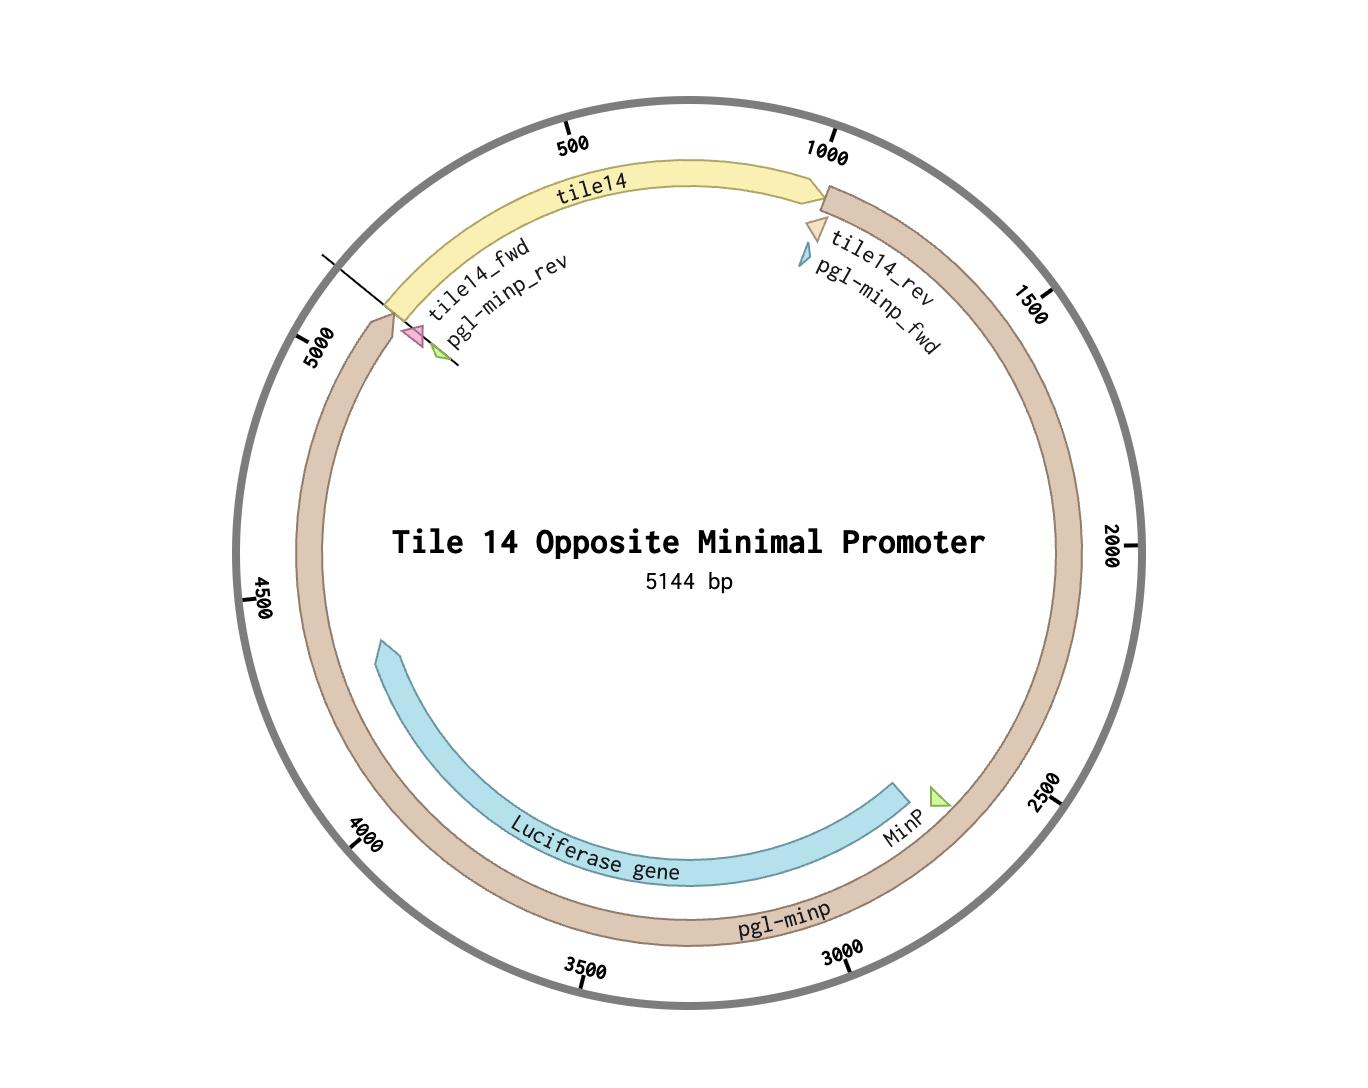
Figure6:PlasmidconstructswiththepolregionandITEopposite aminimalpromoter.
Theseresultshaveimplicationsforunderstandingchronic inflammationinHIV.Defectiveprovirusesarethoughtto contributetochronicinflammationthroughmultiplepathways, includingthroughservingaspathogen-associatedmolecular pathwaysthatactivatepathogenrecognitionreceptors; upregulatingtranscriptionofhumanendogenousretroviruses;and lackingmechanismstoevadeimmuneresponsesinmyeloidcells (Kilroyetal.,2024).Intragenictranscriptionalregulationprovides anewmechanismforunderstandingtheaccumulationofdefective proviraltranscriptsthatcontributetochronicinflammation.For example,perhapsdefectiveprovirusesgeneratedfromintragenic transcriptionalactivityincreaseactivationofpathogenrecognition receptorsinhostcells.Additionally,abnormalsplicingofdefective transcriptscouldtriggerspecificimmuneresponsesevadedby intacttranscripts.Intragenictranscriptionalactivitythus illuminatespossiblenewpathwaysdrivingchronicimmune activationinHIVinfection.SinceU5deficienttranscriptswere
previouslyidentifiedinpeoplelivingwithHIV,thisinvitro understandingofITE-driventranslationcantranslatetoclinical understandingofchronicinflammation(Kuniholmetal.,2021). Furthermore,theITEmayalsoplayaroleinupregulatingnormal HIVtranscriptionthatcontributestopersistentlow-levelimmune activationinpeoplelivingwithHIV.Thus,furthercharacterizing theITEisessentialforunderstandingHIVbiochemistryand pathology.
Conclusion
Theenvelope-regionITEincreasesluciferaseexpression comparedtocontrolsequenceswhenclonedinfrontofaminimal promoterandluciferasereportergene,indicatingthatitbehavesas anintragenicenhancer.Futureexperimentstocharacterizethis activityincludeassayswheretheITEisclonedoppositetoor downstreamofaminimalpromoter.Furthermore,chromatin immunoprecipitationcouldbeusedtocorrelateITEactivitywith levelsofbothintactanddefectiveproviraltranscriptsin HIV-infectedcells.Theseexperimentswouldprovideafoundation forbetterunderstandingITEenhanceractivity,includingitsrolein generatingbothintactanddefectiveviraltranscripts.Theenhancer activitypreliminarilyidentifiedinthispaperprovidesapotential newmechanismforunderstandingchronicinflammationinHIV;it ispossiblethat,throughgenerationofintactanddefectiveproviral transcripts,ITEenhanceractivitytriggersimmuneresponsesthat ultimatelycontributetochronicinflammation.Understanding chronicinflammationmechanismsinHIVisessentialasART continuestoextendthelifeexpectancyofpeoplelivingwithHIV. Characterizingthepathwaysbehindinflammatoryresponsescould eventuallyilluminatewaystopreventortreatHIV-associated chronicinflammatoryconditions.
Bibliography
Abutaleb,A.,&Feinstein,M.(n.d.). Coronary Artery Disease in HIV.AmericanCollegeofCardiology.RetrievedJuly26, 2025,from
https://www.acc.org/Latest-in-Cardiology/Articles/2018/01/ 18/08/57/http%3a%2f%2fwww.acc.org%2fLatest-in-Cardi ology%2fArticles%2f2018%2f01%2f18%2f08%2f57%2fC oronary-Artery-Disease-in-HIV
Akiyama,H.,Jalloh,S.,Park,S.,Lei,M.,Mostoslavsky,G.,& Gummuluru,S.(2021).ExpressionofHIV-1 Intron-ContainingRNAinMicrogliaInducesInflammatory Responses. Journal of virology, 95(5),e01386-20. https://doi.org/10.1128/JVI.01386-20
Boccara,F.,Mary-Krause,M.,Teiger,E.,Lang,S.,Lim,P.,Wahbi, K.,Beygui,F.,Milleron,O.,Steg,P.G.,Funck-Brentano, C,.Slama,M.,Girard,P-M.,Costagliola,D.,Cohen,A. Acutecoronarysyndromeinhumanimmunodeficiency virus-infectedpatients:Characteristicsand1year prognosis. European Heart Journal, 32(1). https://doi.org/10.1093/eurheartj/ehq372
Burdo,T.H.,Weiffenbach,A.,Woods,S.P.,Letendre,S.,Ellis,R. J.,&Williams,K.C.(2013).ElevatedsCD163inplasma butnotcerebrospinalfluidisamarkerofneurocognitive impairmentinHIVinfection. AIDS (London, England), 27(9),1387–1395. https://doi.org/10.1097/QAD.0b013e32836010bd CentersforDiseaseControlandPrevention.(1982).Updateon acquiredimmunedeficiencysyndrome(AIDS)—United States. MMWR. Morbidity and Mortality Weekly Report, 31(37),507–508,513–514.
DavidJ.SencerCDCMuseum. The AIDS Epidemic in the United States, 1981-early 1990s.(2024).RetrievedAugust8,
2025,from https://www.cdc.gov/museum/online/story-of-cdc/aids/inde x.html
Drozd,D.R.,Kitahata,M.M.,Althoff,K.N.,Zhang,J.,Gange,S. J.,Napravnik,S.,Burkholder,G.A.,Mathews,W.C., Silverberg,M.J.,Sterling,T.R.,Heckbert,S.R.,Budoff, M.J.,VanRompaey,S.,Delaney,J.A.C.,Wong,C.,Tong, W.,Palella,F.J.,Elion,R.A.,Martin,J.N.,…Crane,H. M.(2017).IncreasedRiskofMyocardialInfarctionin HIV-InfectedIndividualsinNorthAmericaComparedWith theGeneralPopulation. JAIDS Journal of Acquired Immune Deficiency Syndromes, 75(5),568. https://doi.org/10.1097/QAI.0000000000001450
JointUnitedNationsProgrammeonHIV/AIDS. Global HIV & AIDS statistics.(n.d.).RetrievedAugust23,2025,from https://www.unaids.org/en/resources/fact-sheet
JointUnitedNationsProgrammeonHIV/AIDS. Impact of US funding cuts on the global HIV response (2025).Retrieved January8,2026,from https://www.unaids.org/en/impact-US-funding-cuts/About Kilroy,J.M.,Leal,A.A.,&Henderson,A.J.(2024).ChronicHIV Transcription,Translation,andPersistentInflammation. Viruses, 16(5),751.https://doi.org/10.3390/v16050751
Krebs,F.C.,Hogan,T.H.,Quiterio,S.J.,Gartner,S.,&Wigdahl,B. (2002).LentiviralLTR-directedExpression, Sequence Variation,andDiseasePathogenesis. Los Alamos National Laboratory.
https://www.hiv.lanl.gov/content/sequence/HIV/COMPEN DIUM/2001/partI/Wigdahl.pdf
Kuniholm,J.,Armstrong,E.,Bernabe,B.,Coote,C.,Berenson,A., Patalano,S.D.,Olson,A.,He,X.,Lin,N.H.,Bass,J.I.F., &Henderson,A.J.(2021).Intragenicproviralelements
supporttranscriptionofdefectiveHIV-1proviruses. PLOS Pathogens, 17(12),e1009982.
https://doi.org/10.1371/journal.ppat.1009982
LosAlamosNationalLaboratory. Landmarks of the HIV genome. (n.d.).RetrievedAugust13,2025,from https://www.hiv.lanl.gov/content/sequence/HIV/MAP/land mark.html
NationalInstituteofAllergyandInfectiousDiseases. Antiretroviral Drug Discovery and Development. (n.d.).
RetrievedJuly15,2025,from https://oar.nih.gov/about/history/oar-35-years
NewEnglandBiolabs. Ligation Protocol with T4 DNA Ligase (M0202) | NEB.(n.d.).RetrievedJuly17,2025,from https://www.neb.com/en-us/protocols/0001/01/01/dna-ligati on-with-t4-dna-ligase-m0202
NewEnglandBiolabs. PCR Using Q5® High-Fidelity DNA Polymerase (NEB #M0491) | NEB.(n.d.).RetrievedJuly 18,2025,from https://www.neb.com/en-us/protocols/2013/12/13/pcr-using -q5-high-fidelity-dna-polymerase-m0491
NewEnglandBiolabs. Restriction Enzyme Double Digestion. (n.d.).NEBcloner.RetrievedJuly17,2025,from https://nebcloner.neb.com/#!/protocol/re/double/SacI-HF,X hoI
Peruski,A.H.,Wesolowski,L.G.,Delaney,K.P.,Chaves,P.R., Owen,S.M.,Granade,T.C.,Sullivan,V.,Switzer,W.M., Dong,X.,Brooks,J.T.,&Joyce,P.M.(2020).Trendsin HIV-2DiagnosesandUseoftheHIV-1/HIV-2 DifferentiationTest—UnitedStates,2010–2017. MMWR. Morbidity and Mortality Weekly Report, 69. https://doi.org/10.15585/mmwr.mm6903a2
Promega. Dual-Glo® Luciferase Assay System Technical Manual. (n.d.).RetrievedJuly18,2025,from https://www.promega.com/products/luciferase-assays/repor ter-assays/dual_glo-luciferase-assay-system/ Promega. Minimal Promoter-Driven Firefly Luciferase Vectors. (n.d.).RetrievedJuly14,2025,from https://www.promega.com/products/luciferase-assays/genet ic-reporter-vectors-and-cell-lines/minimal-promoter-driven -firefly-luciferase-vectors/ Ramaswamy,S.,Akiyama,H.,Berrigan,J.,Quiñones-Molina,A. A.,Olson,A.J.,Chen,Y.,Liang,Y.,Henderson,A.J., Asundi,A.,Sagar,M.,&Gummuluru,S.(2025).The macrophage-intrinsicMDA5/IRF5axisdrivesHIV-1 intron-containingRNA-inducedinflammatoryresponses. The Journal of clinical investigation, 135(16),e187663. https://doi.org/10.1172/JCI187663 Rosenthal,J.,&Tyor,W.(2019).Aging,comorbidities,andthe importanceoffindingbiomarkersforHIV-associated neurocognitivedisorders. Journal of Neurovirology, 25, 673–685.
https://doi-org.ezproxy.bu.edu/10.1007/s13365-019-007350 Rossi,E.,Meuser,M.E.,Cunanan,C.J.,&Cocklin,S.(2021). Structure,Function,andInteractionsoftheHIV-1Capsid Protein. Life, 11(2),100.
https://doi.org/10.3390/life11020100 Schmid,S.(2018).ThediscoveryofHIV-1. Nature Research. https://doi.org/10.1038/d42859-018-00003-x Triant,V.A.,Lee,H.,Hadigan,C.,&Grinspoon,S.K.(2007).
IncreasedAcuteMyocardialInfarctionRatesand CardiovascularRiskFactorsamongPatientswithHuman ImmunodeficiencyVirusDisease. The Journal of Clinical
Endocrinology & Metabolism, 92(7),2506–2512.
https://doi.org/10.1210/jc.2006-2190
Trickey,A.,Sabin,C.A.,Burkholder,G.,Crane,H.,Monforte,A. d’Arminio,Egger,M.,Gill,M.J.,Grabar,S.,Guest,J.L., Jarrin,I.,Lampe,F.C.,Obel,N.,Reyes,J.M.,Stephan,C., Sterling,T.R.,Teira,R.,Touloumi,G.,Wasmuth,J.-C., Wit,F.,…Sterne,J.A.C.(2023).Lifeexpectancyafter 2015ofadultswithHIVonlong-termantiretroviraltherapy inEuropeandNorthAmerica:Acollaborativeanalysisof cohortstudies. The Lancet HIV, 10(5),e295–e307.
https://doi.org/10.1016/S2352-3018(23)00028-0